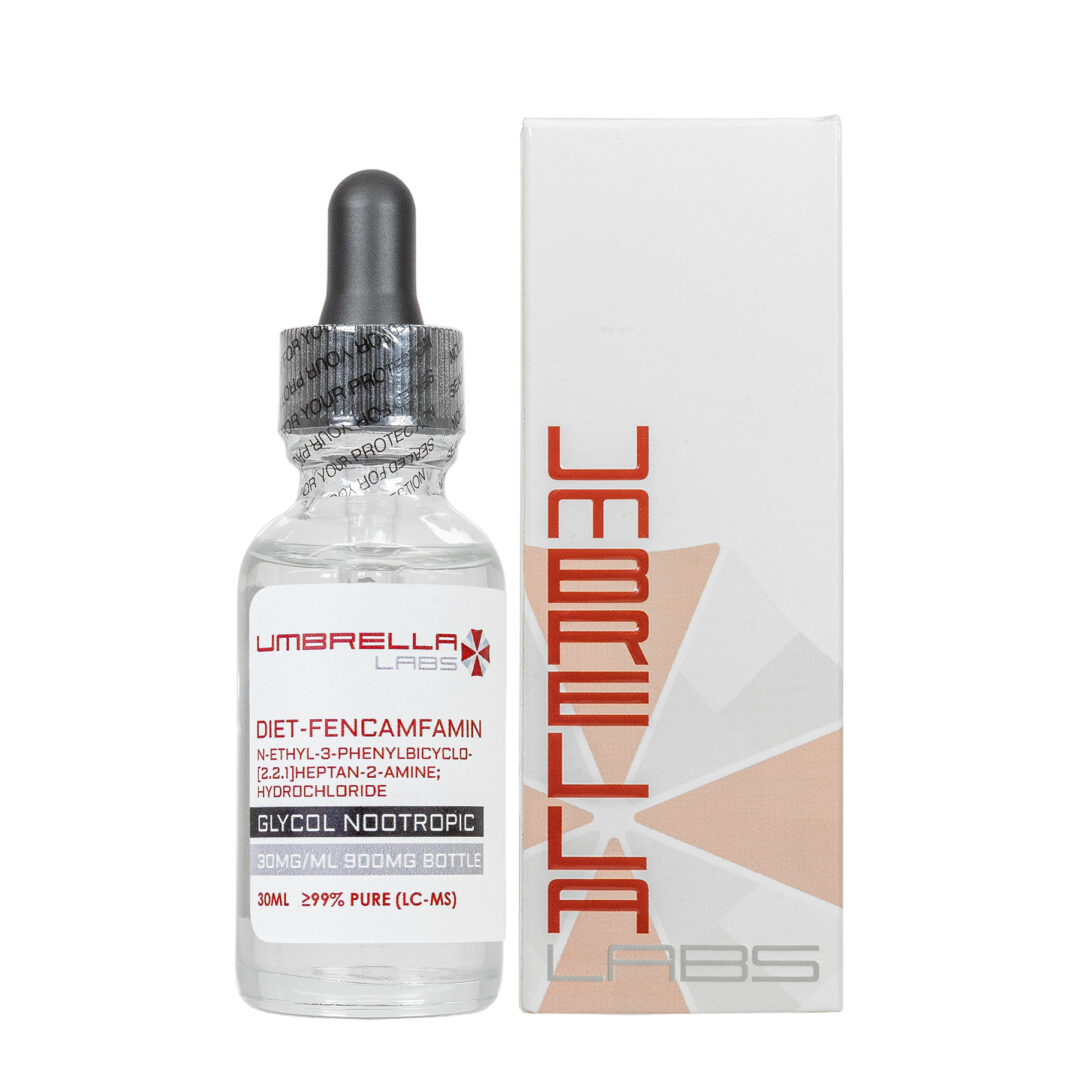
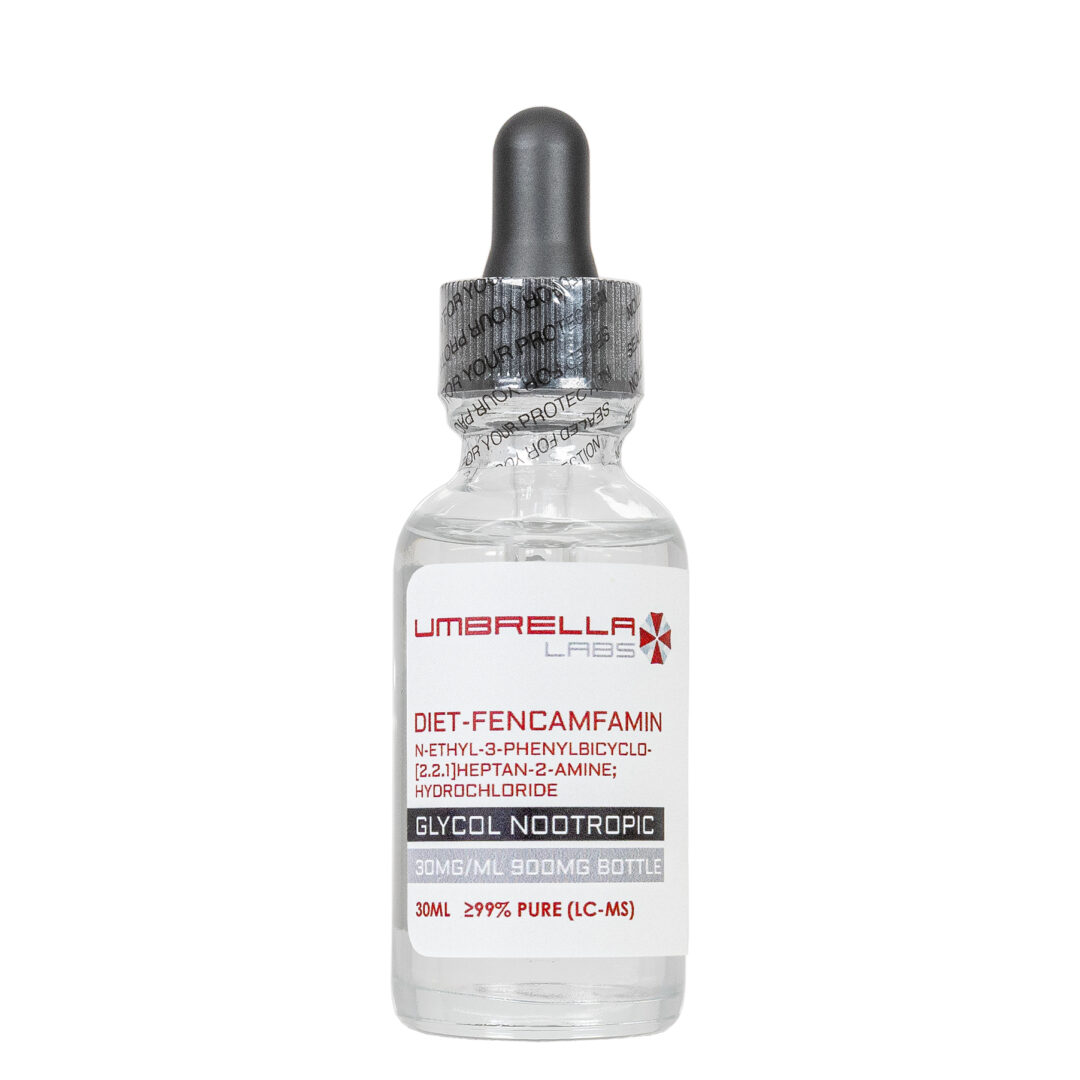
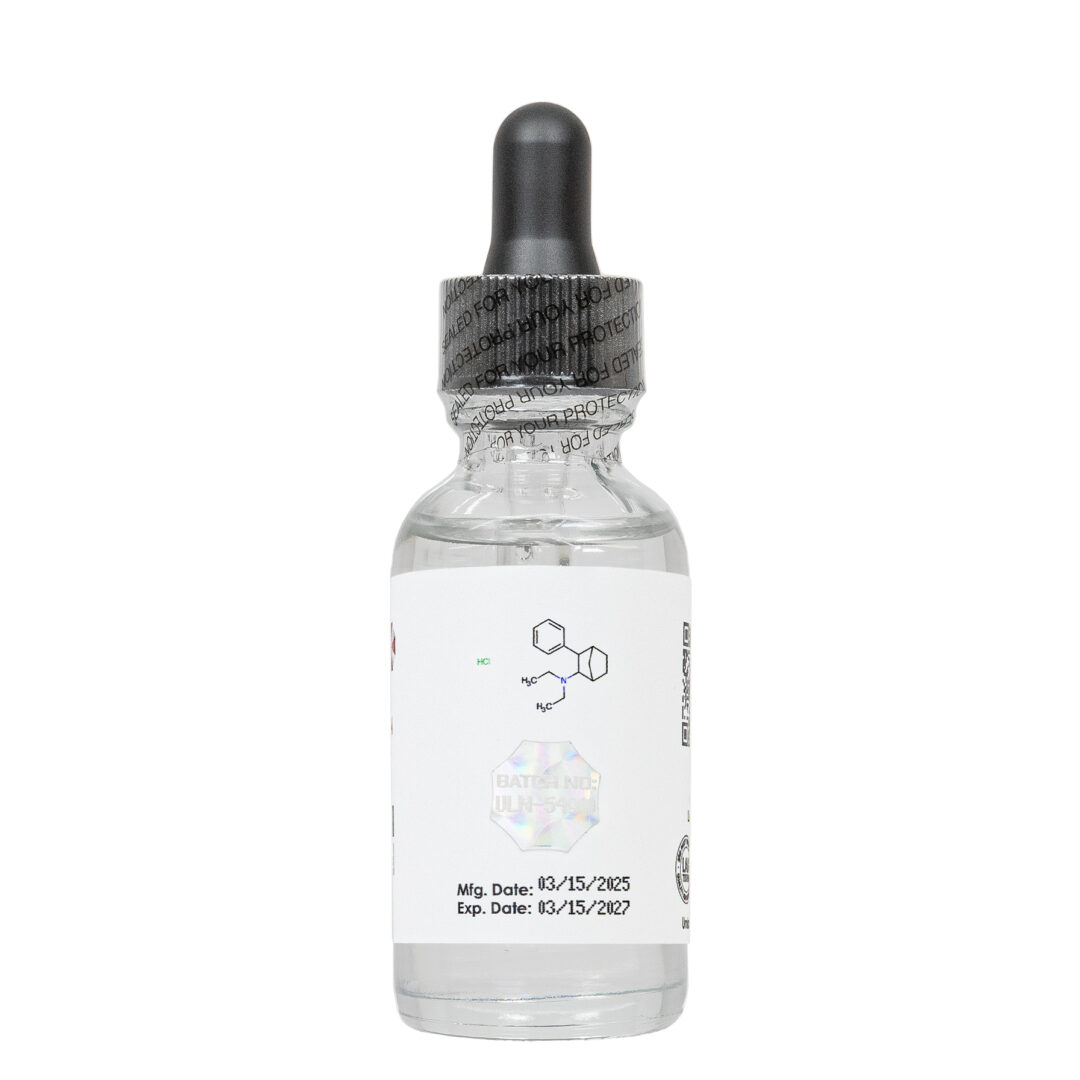
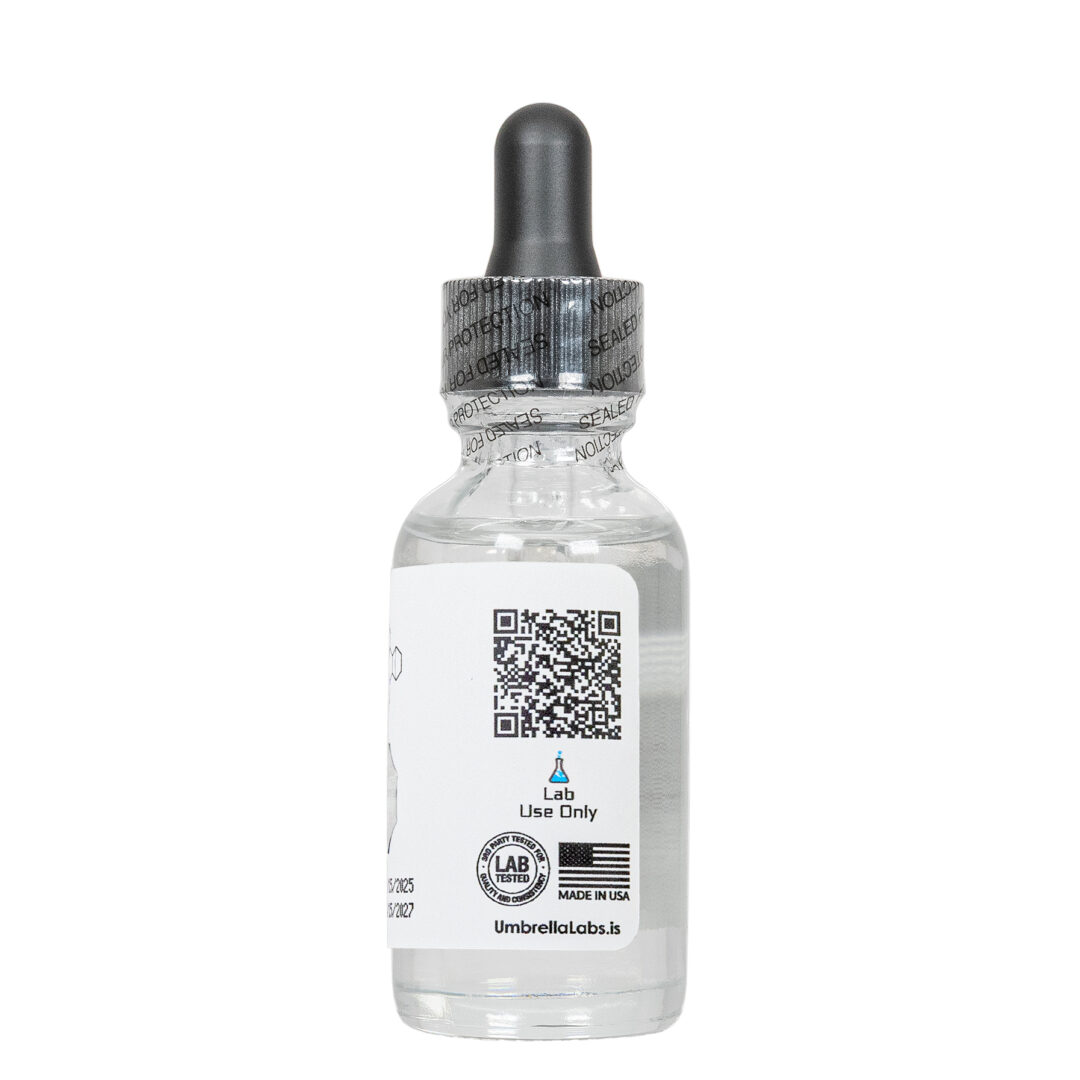
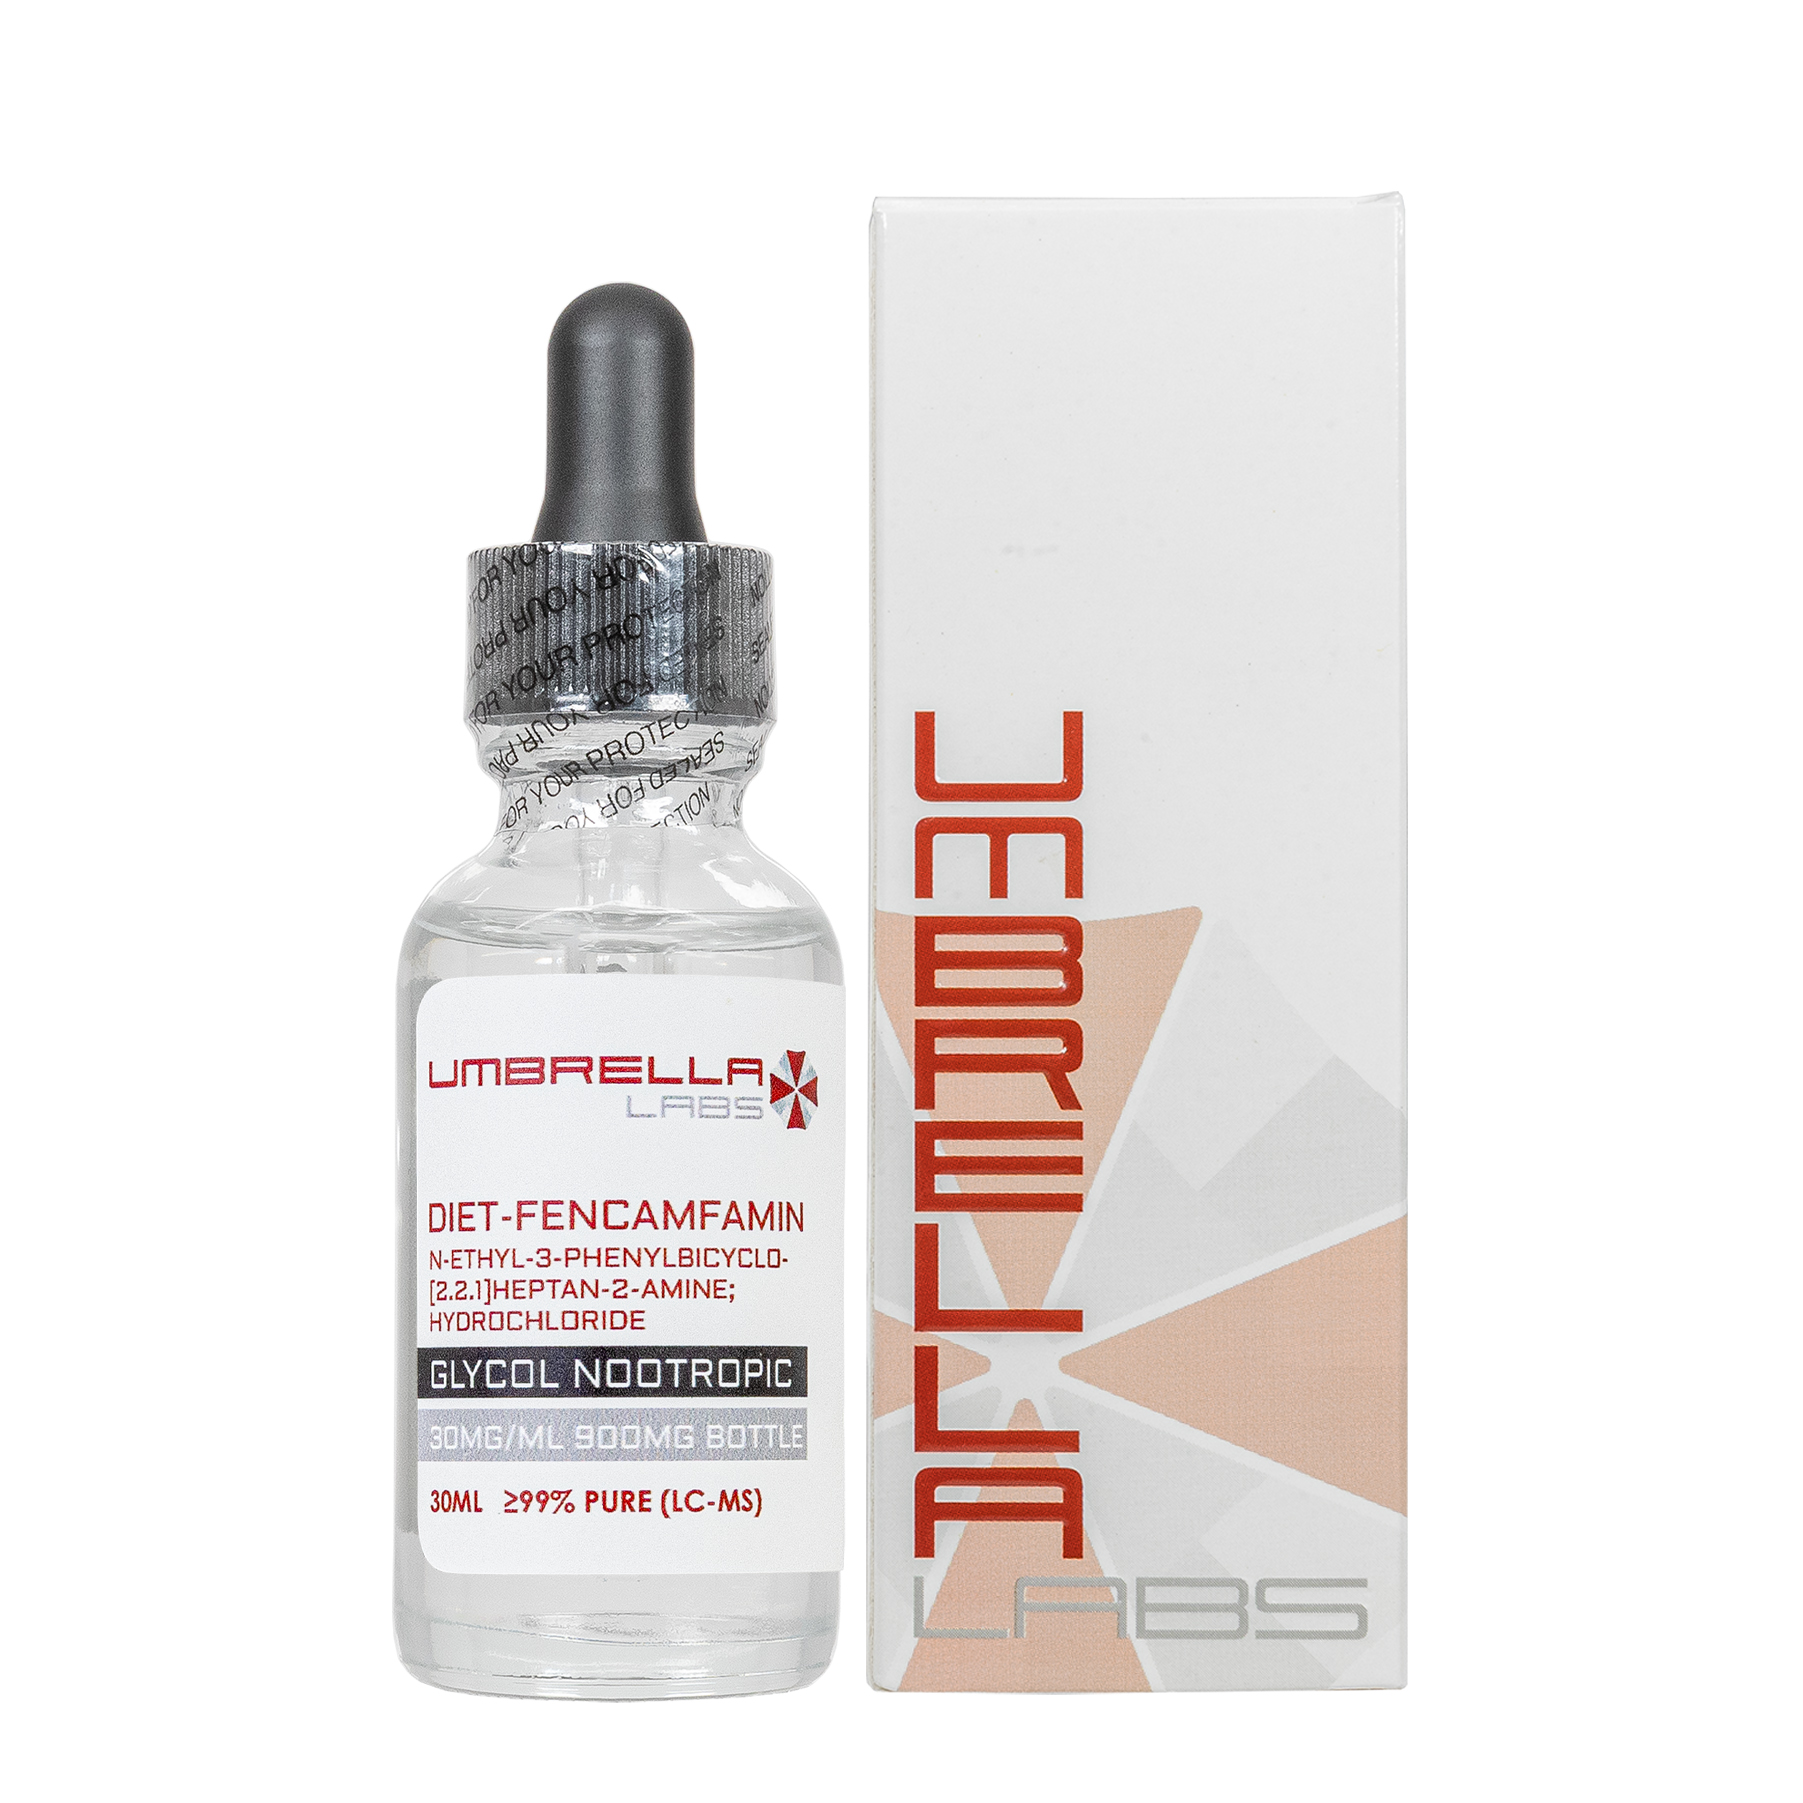
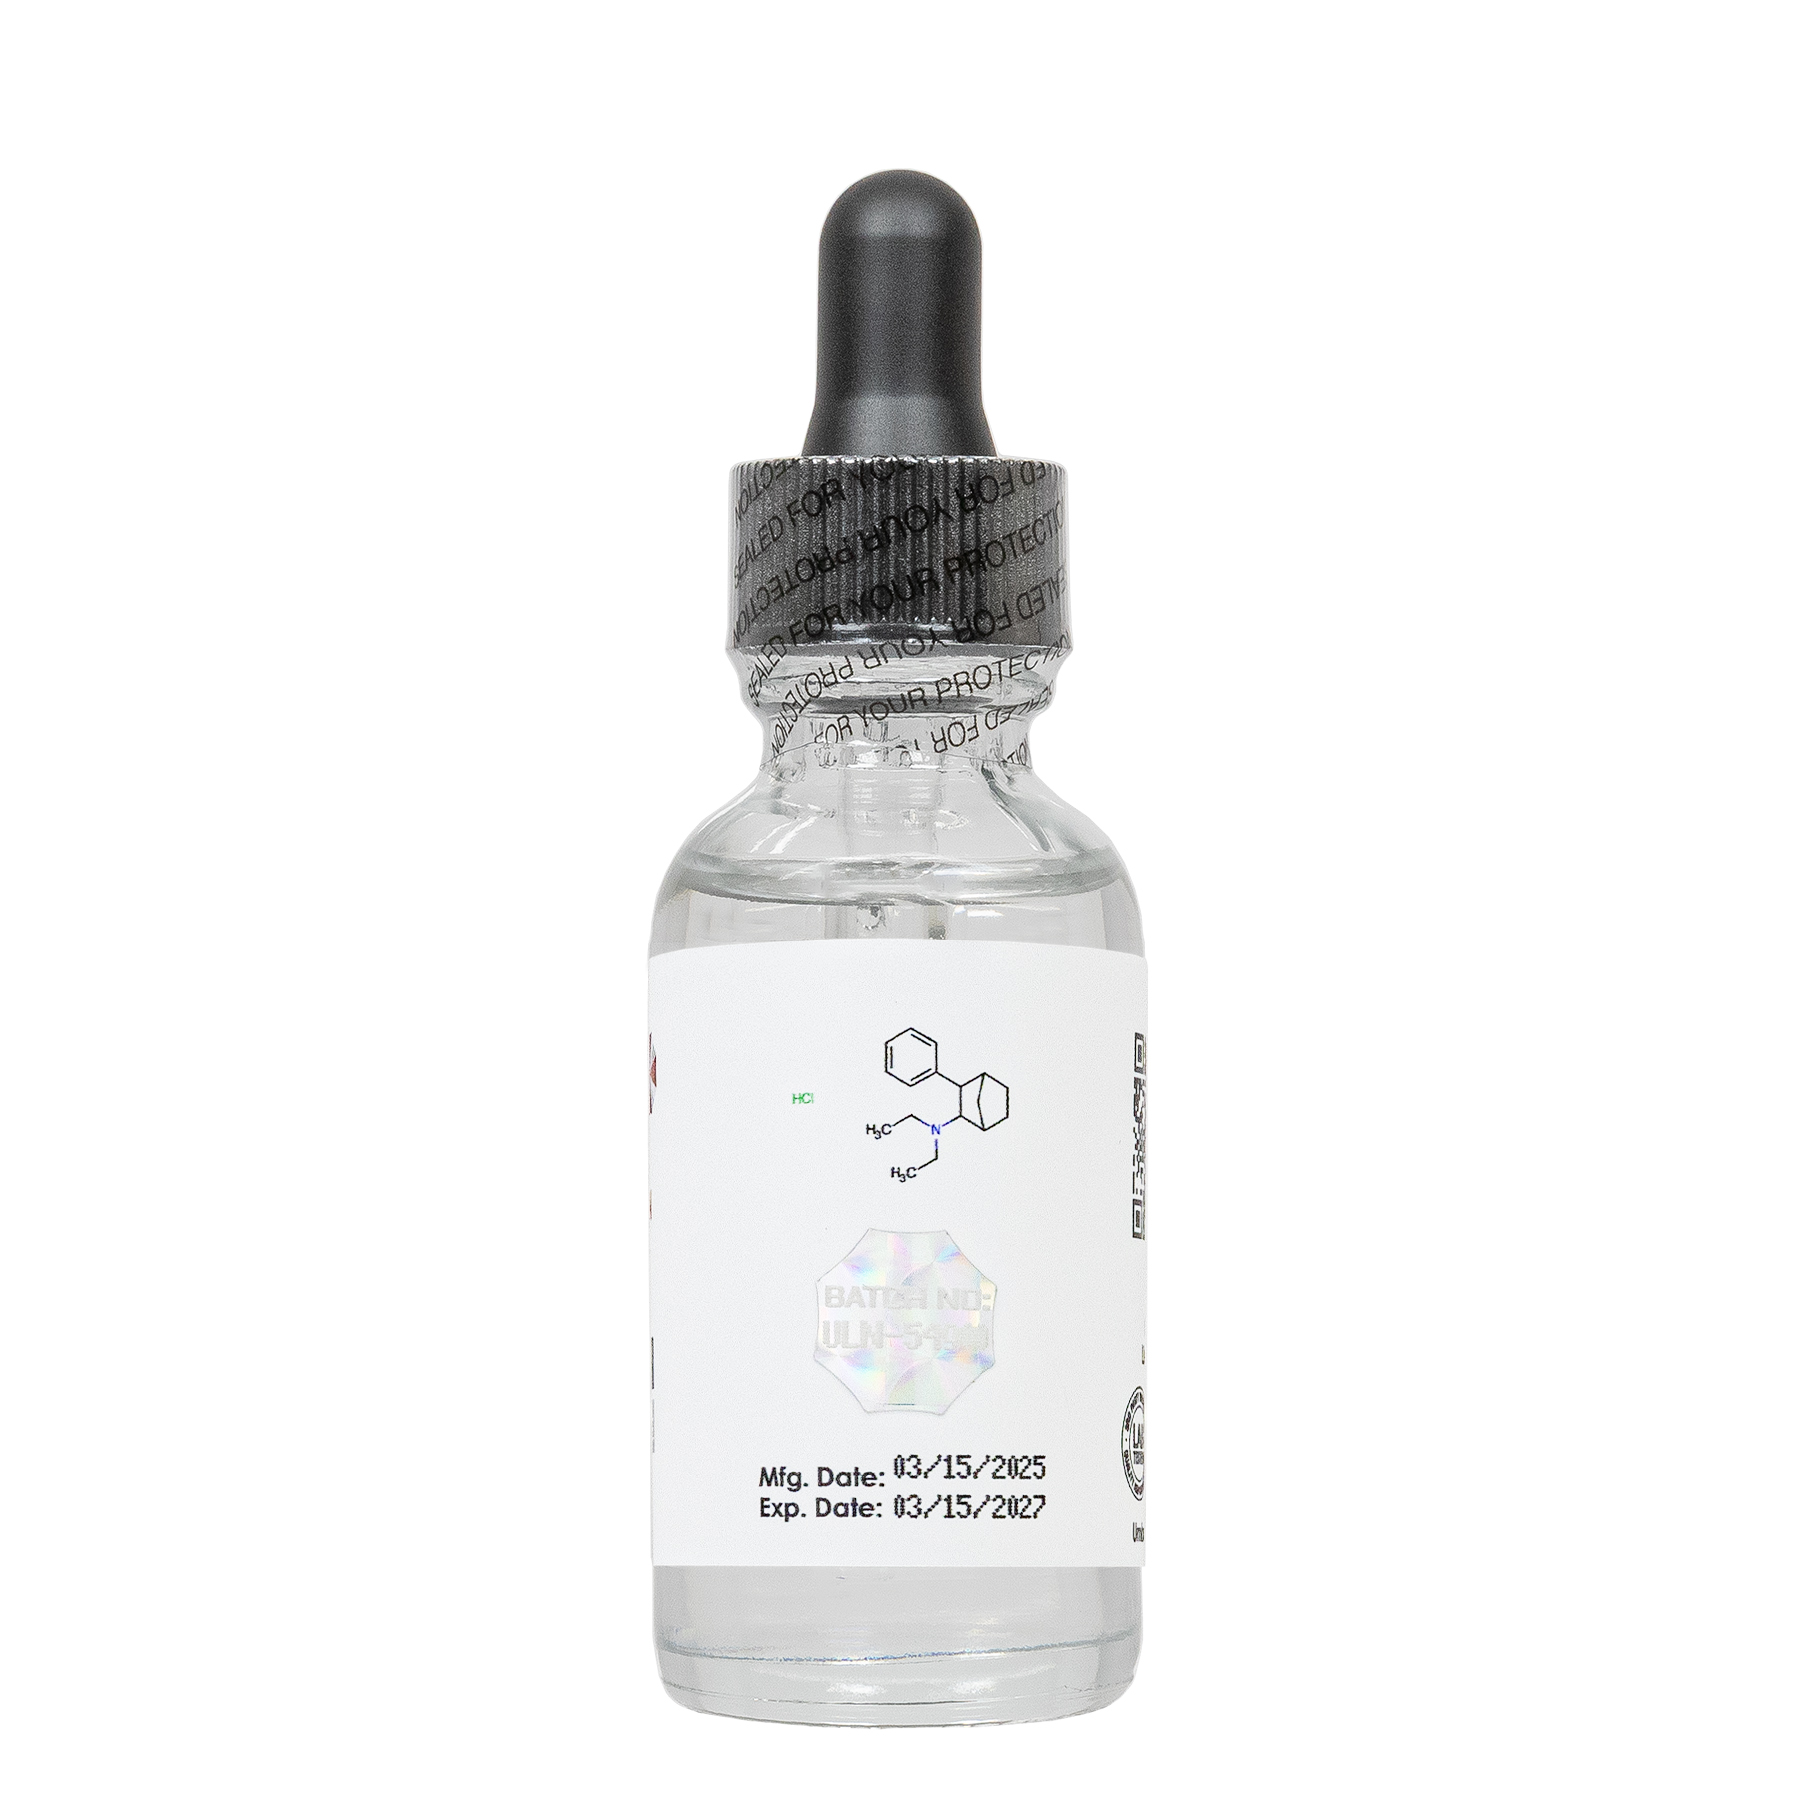
DIET-FENCAMFAMIN 30ML LIQUID (30MG/ML, 900MG BOTTLE)
$129.99
DiEt-Fencamfamin is sold for laboratory research use only. Terms of sale apply. Not for human consumption, nor medical, veterinary, or household uses. Please familiarize yourself with our Terms & Conditions prior to ordering.
- Description
- Additional information
Description
DiEt-Fencamfamin Research Chemical Liquid
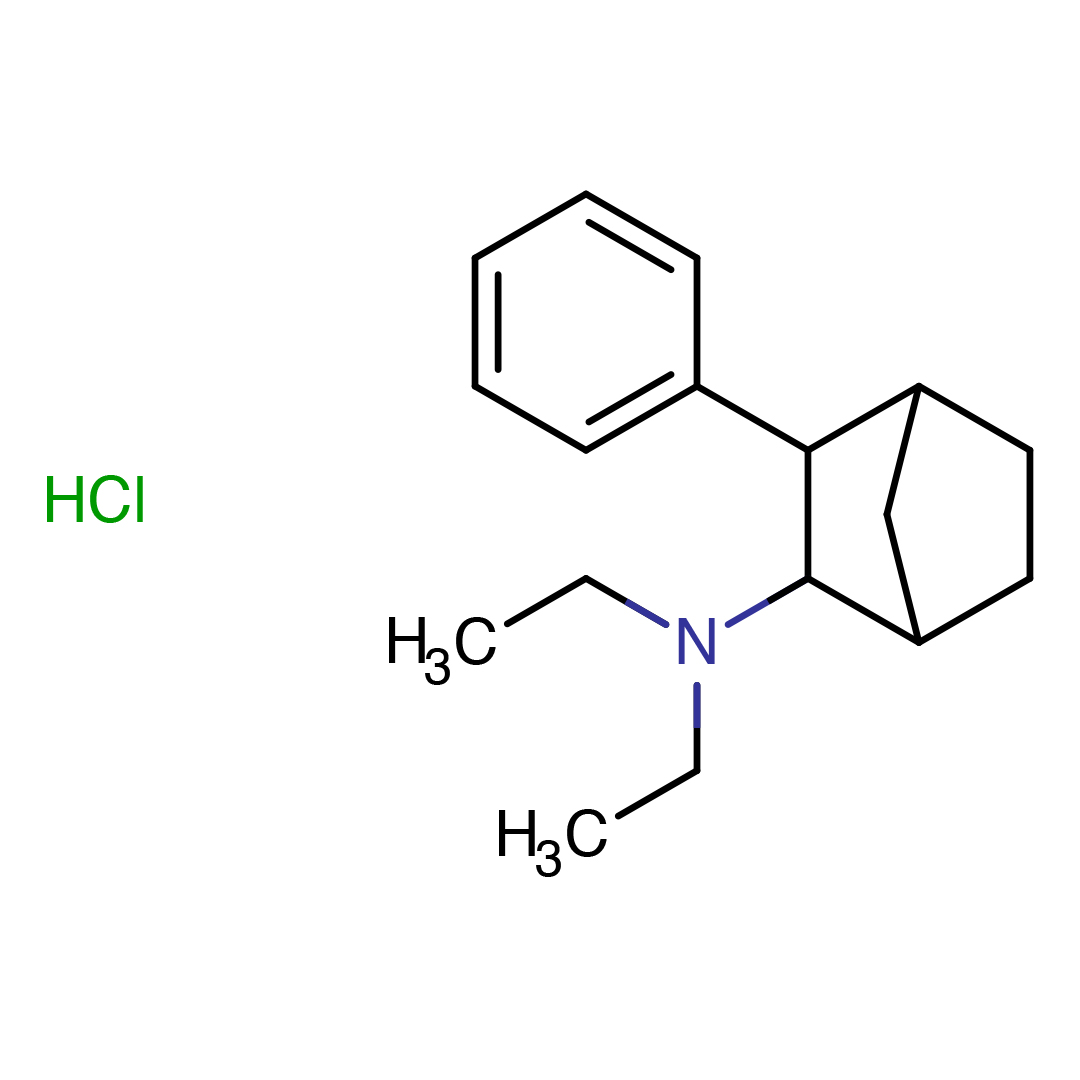
| CAS Number | 7177-30-2 |
| Other Names | DiEt-Fencamfamine HCl, N-Ethylfencamfamine HCl, N-N-diethyl-3-phenyl-2-norbornanamine hydrochloride, N-N-diethyl-3-phenylbicyclo[2.2.1]heptan-2-amine hydrochloride |
| IUPAC Name |
N-ethyl-3-phenylbicyclo[2.2.1]heptan-2-amine;hydrochloride
|
| Molecular Formula | C₁₇H₂₅N•HCl |
| Molecular Weight | 243.39 |
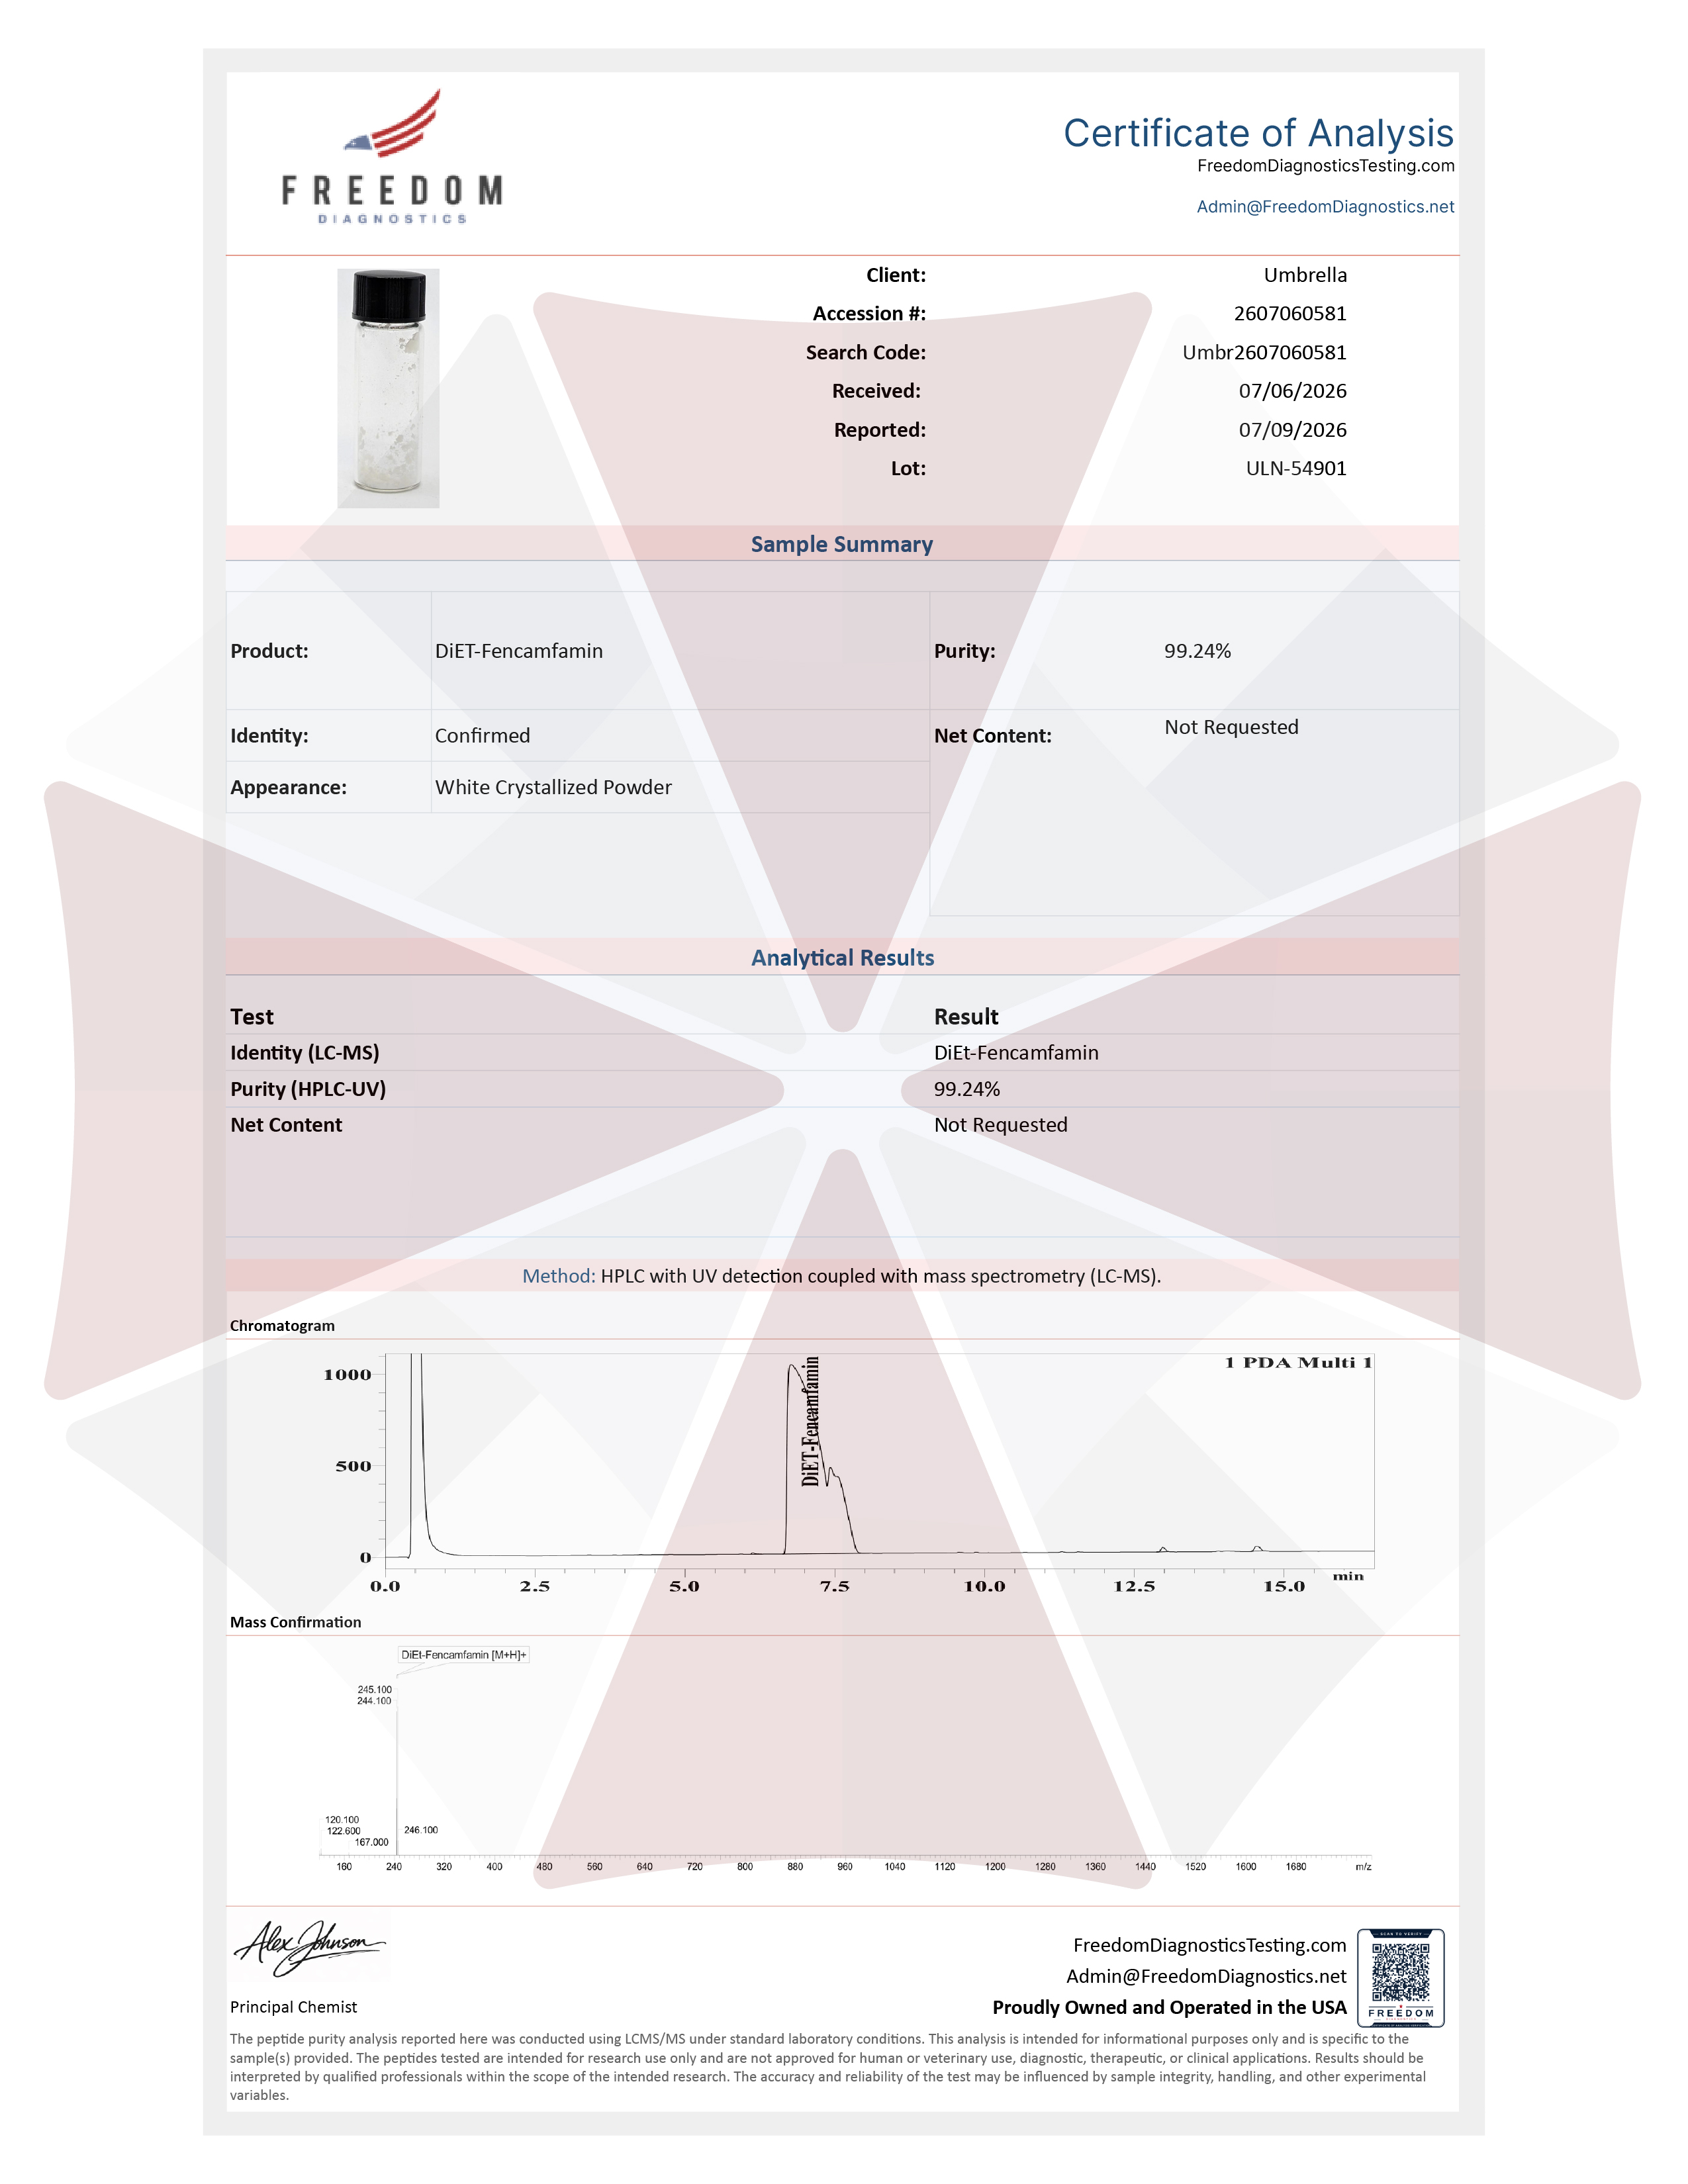
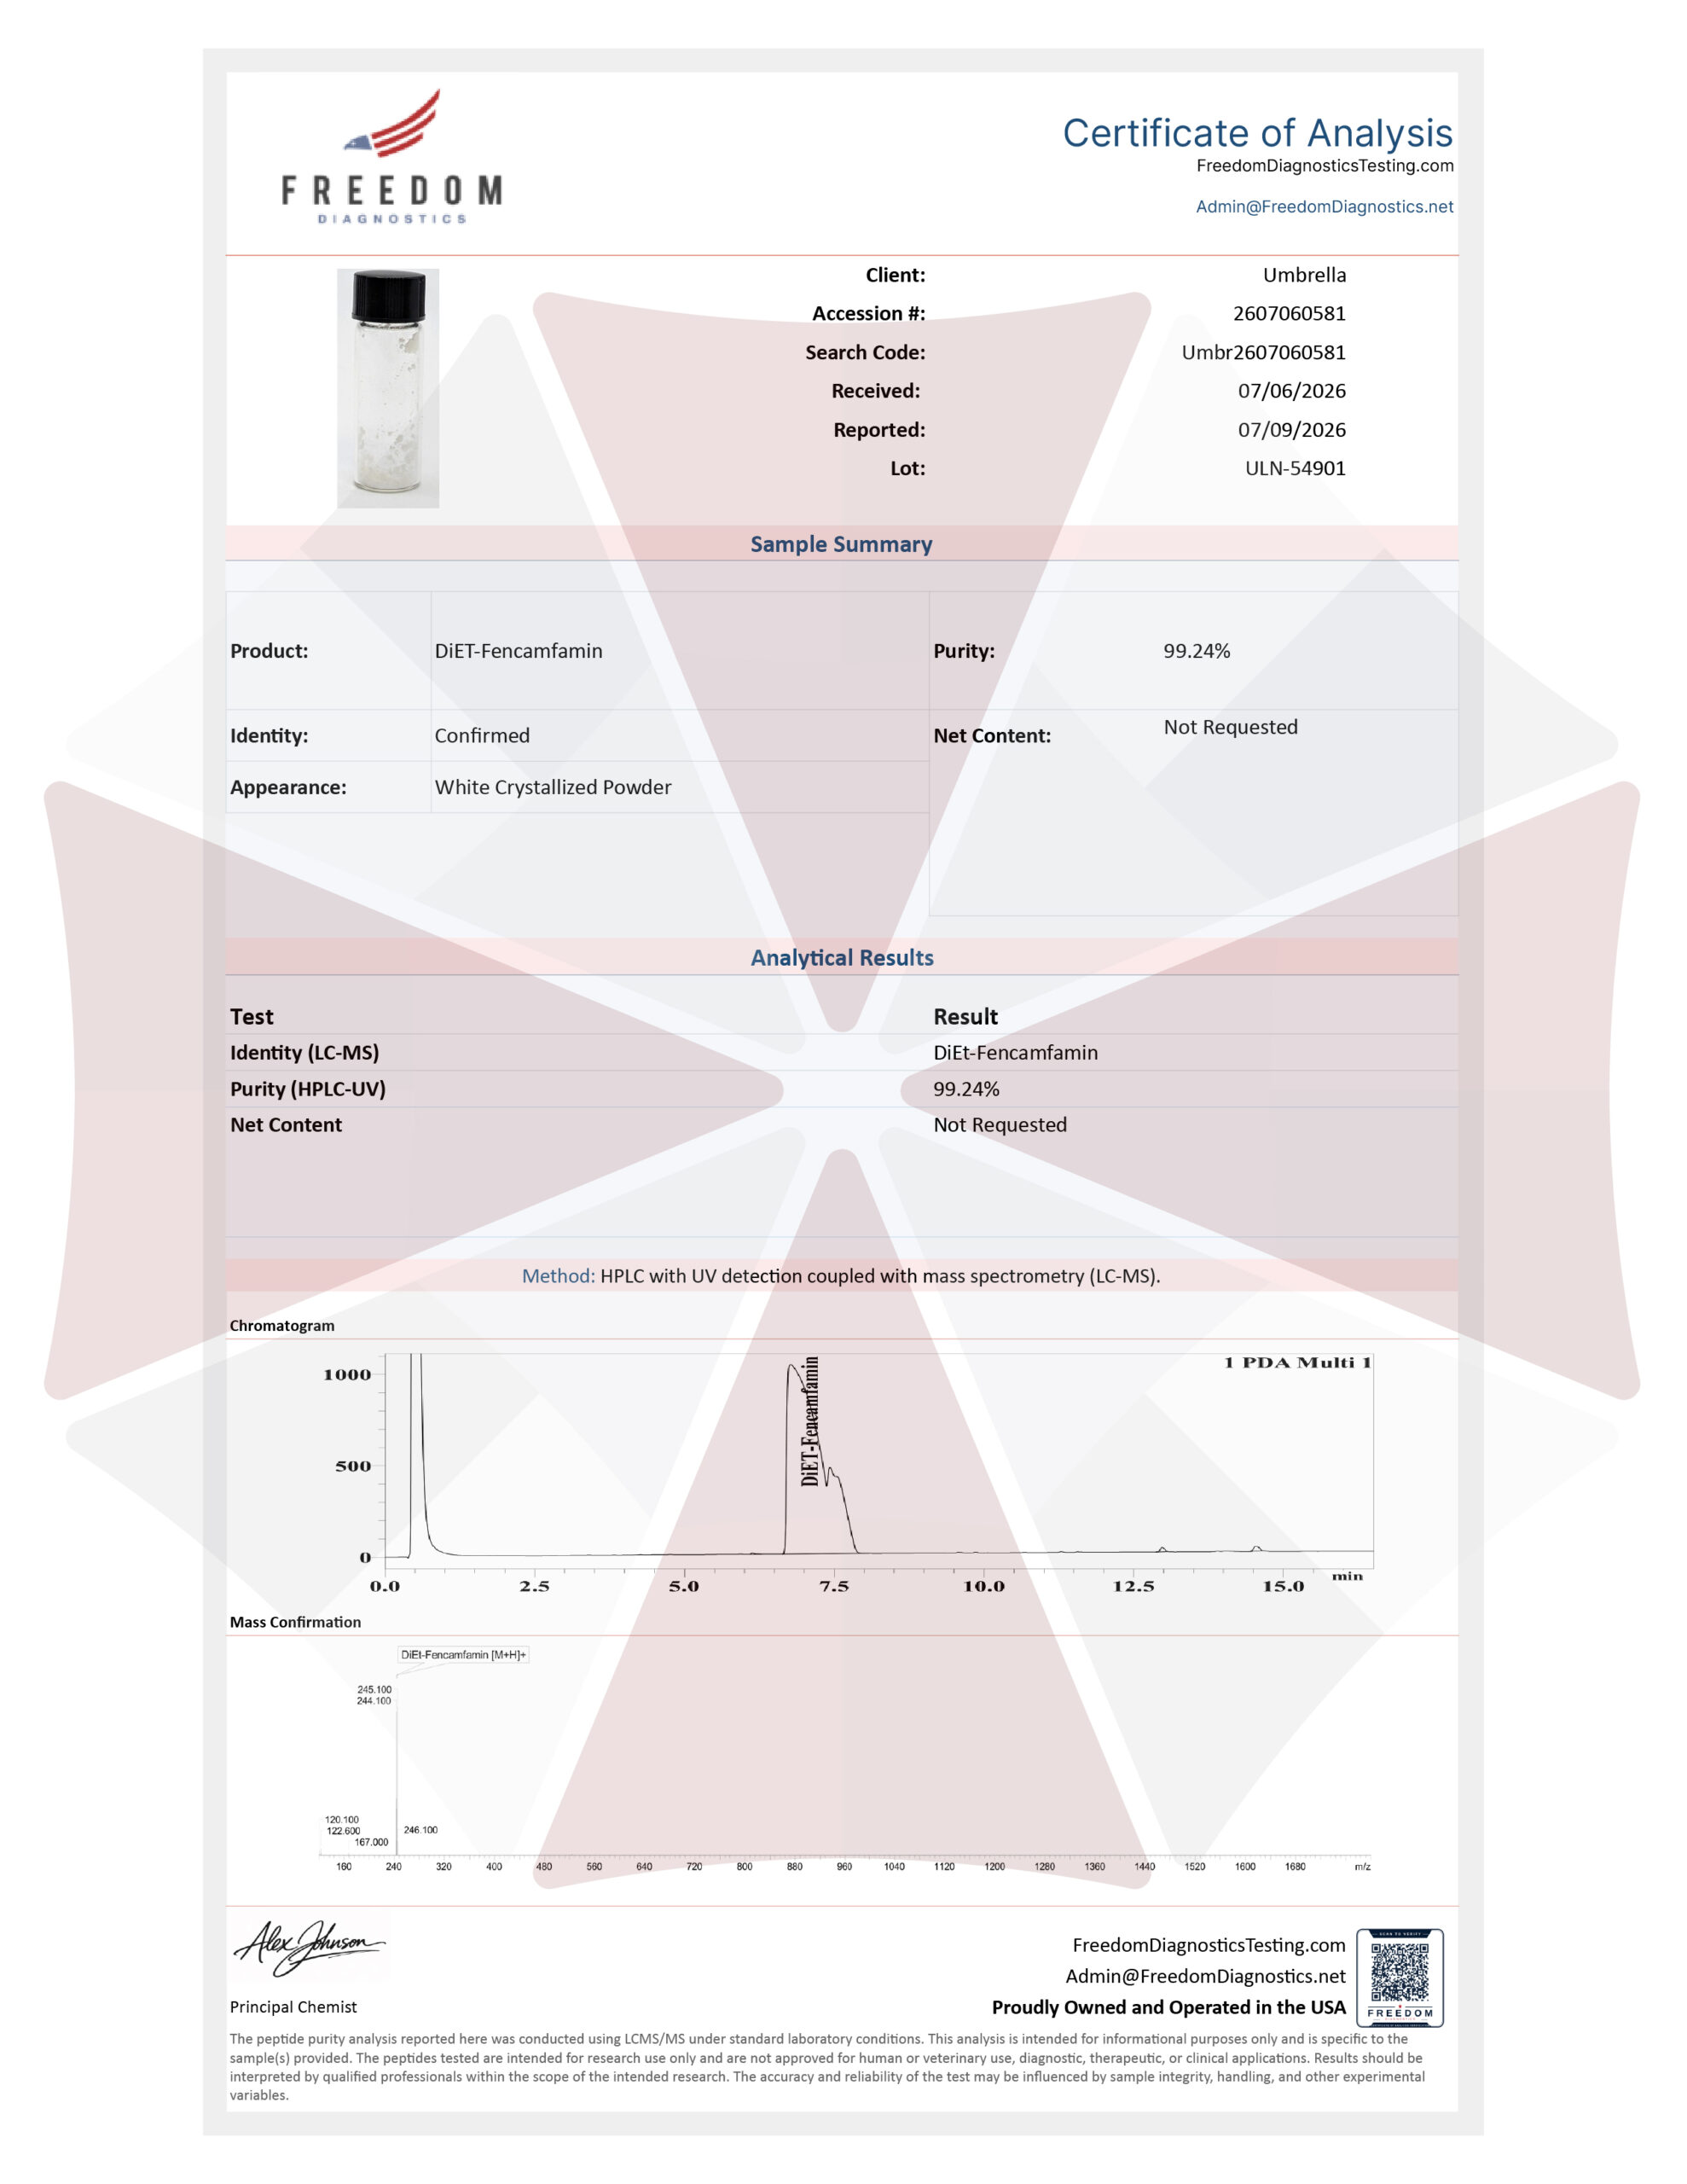
| Purity | ≥99% Pure (LC-MS) |
| Liquid Availability |  30mL Liquid (30mg/mL, 900mg total bottle) |
| Powder Availability | 1 gram
|
| Storage | Store in cool dry environment, away from direct sunlight. |
| Terms | All products are for laboratory developmental research USE ONLY. Products are not for human consumption. |
What is Fencamfamine?
Fencamfamine is a central nervous system stimulant first developed in the 1960s, historically used as an antidepressant, wakefulness aid, and appetite suppressant. It exerts stimulant effects mainly by enhancing dopamine and norepinephrine signaling, which can increase alertness, motivation, and psychomotor performance, qualities of interest for cognitive enhancement.
Main Research Findings
1) Fencamfine was shown to modulate sodium and potassium ATPase through activation of cyclic AMP and cyclic AMP-dependent proteins
2) Repeated administration of Fencamfamine was found to intensify the place-preference, reinforcing, and rewarding effects of the compound.
Selected Data
1) This study completed by the research team of Ferreira et al investigated how FCF, a psychostimulant with dopaminergic activity, modulates Na⁺/K⁺-ATPase activity in the rat striatum, and whether this modulation occurs through cyclic AMP (cAMP) and protein kinase signaling pathways. To achieve this, the researchers designed a series of biochemical experiments using isolated rat brain tissue and pharmacological manipulations [1].
Male Wistar rats weighing between 350–400 grams were used as the experimental model. The animals were euthanized via decapitation under ether anesthesia to minimize distress and preserve brain tissue integrity. Immediately after sacrifice, the brains were removed, and the striatum, a brain region heavily involved in dopaminergic signaling, was carefully dissected. The striatal tissue was then sectioned into small slices measuring 0.3 × 0.3 × 1 mm, using a mechanical tissue chopper. These slices were washed thoroughly to remove debris and maintained at 4°C before being resuspended in a physiological buffer solution. This buffer contained key ions, NaCl, KCl, MgSO₄, CaCl₂, and HEPES to maintain pH at 7.4, approximating physiological conditions [1].
To assess enzyme activity, the researchers employed a permeabilized slice technique. Tissue slices were treated with freezing and thawing steps followed by incubation with alamethicin, a detergent that permeabilizes cell membranes without disrupting enzyme function. This ensured that ATP and other substrates could freely access intracellular enzymes. The ATPase activity assay relied on measuring the hydrolysis of radiolabeled ATP (γ-³²P-ATP). After incubation, the amount of inorganic phosphate (³²Pi) released from ATP hydrolysis was quantified using scintillation counting. This provided a direct measure of ATPase activity.
To distinguish Na⁺/K⁺-ATPase activity from other ATPases, such as Mg-ATPase, the researchers used ouabain, a specific inhibitor of Na⁺/K⁺-ATPase. By comparing total ATPase activity (without ouabain) to ouabain-insensitive activity (with ouabain), they calculated the specific Na⁺/K⁺-ATPase component. Protein content in each sample was measured using a colorimetric assay, allowing enzyme activity to be normalized per milligram of protein. Under the assay conditions, substrate concentrations were saturating, ensuring maximal enzyme activity and reliable comparisons.
A variety of pharmacological agents were used to probe the mechanism of FCF action. First, FCF was tested at concentrations ranging from 10 to 100 µM to establish dose-response effects. Dopamine (DA) was used at 10 µM as a comparison, since FCF is known to influence dopaminergic signaling. 8-बromo-cAMP, is a membrane-permeable analog of cAMP used to mimic intracellular cAMP signaling. Dopamine receptor antagonists including SCH 23390 and Sulpiride were used as D1 and D2 receptor antagonists, respectively. Finally, protein kinase inhibitor KT 5720 was used as a selective inhibitor of protein kinase A, PKA and protein kinase inhibitor KT 5823 was used as a selective inhibitor of protein kinase G, PKG [1].
Drugs were added to striatal slice suspensions and incubated under controlled conditions. In some experiments, tissues were pretreated with receptor antagonists or kinase inhibitors before exposure to FCF or other agents. Each experimental condition included multiple replicates of five samples per condition, and experiments were repeated independently to ensure reproducibility.
To evaluate whether FCF influences intracellular signaling pathways, levels of cyclic nucleotides, cAMP and cGMP, were measured using radioimmunoassay techniques. After drug treatment, supernatants from slice suspensions were collected and chemically processed to enhance assay sensitivity. Samples were acetylated and heated before being subjected to radioimmunoassay using commercially available kits. This allowed precise quantification of intracellular cAMP and cGMP concentrations.
The study included several key comparisons including dose-response effects of FCF on ATPase activity, the effects between FCF and dopamine, the combined treatment with FCF and dopamine to test for additive or shared mechanisms, the effects of receptor blockade D1 and D2 antagonists, the effects of kinase inhibition through PKA vs PKG, and the use of cAMPT analogs to mimic intracellular signaling. Control groups included untreated slices and slices treated with inhibitors alone to ensure that observed effects were specific to the experimental manipulations [1].
2) This study performed by the research team of DeLucia et al describes the experimental methods used to investigate the behavioral and rewarding effects of FCF in rats, with a particular focus on sensitization following repeated drug exposure. The study used controlled laboratory conditions, well-defined behavioral measurements, and established experimental paradigms to evaluate both locomotor activity and drug-associated reward.
The subjects in this study were adult male Wistar rats weighing between 250 and 300 grams. These animals were housed under standardized environmental conditions to ensure consistency across experiments. Specifically, they were maintained at a temperature of 22 ± 2°C and kept on a 12-hour light/12-hour dark cycle, with lights turning on at 7:00 AM. This light-dark cycle was maintained for nine weeks prior to the start of the experiments, allowing the animals to fully acclimate to their environment. Food and water were available to the rats at all times, except during behavioral observation periods when both were temporarily removed to avoid interference with activity measurements. All behavioral testing was conducted during the light phase of the cycle to maintain consistency in circadian influences on activity [2].
Fencamfamine hydrochloride, the drug of interest, was obtained from Merck and prepared in a 0.9% saline solution. It was administered intraperitoneally at a volume of 1 ml/kg, and all doses were expressed based on the weight of the salt form of the drug. Saline injections were used as a control condition to compare against the effects of FCF. The study consisted of two main experiments designed to examine different aspects of drug sensitization. Experiment I focused on behavioral sensitization, which refers to the progressive increase in a drug’s effects following repeated exposure. Experiment II examined sensitization to the rewarding properties of the drug using a conditioned place preference (CPP) paradigm [2].
In Experiment I, a total of 16 rats were divided into two groups of eight animals each. One group received daily injections of FCF at a dose of 3.5 mg/kg, while the other group received saline injections. These treatments were administered intraperitoneally once per day for ten consecutive days. After the final injection, the rats were observed in their home cages to assess behavioral changes. Behavioral observations began 30 minutes after the last injection. The researchers measured three specific behaviors: locomotion, rearing, and sniffing. Locomotion was defined as movement involving all four legs, rearing as standing with both front feet off the ground, and sniffing as exploratory behavior with all feet remaining on the cage floor. These behaviors were recorded for 60 seconds at 15-minute intervals over a total observation period of 90 minutes. Importantly, the observer recording these behaviors was blind to the treatment conditions, reducing the risk of bias in the data collection process. This design allowed the researchers to determine whether repeated FCF administration led to enhanced behavioral responses indicative of sensitization.
Experiment II used another group of 16 rats, again divided into two groups of eight, to evaluate the rewarding effects of FCF through a conditioned place preference procedure. As in the first experiment, rats received daily injections of either FCF (3.5 mg/kg) or saline for ten consecutive days. However, instead of observing spontaneous behavior, this experiment paired drug administration with a specific environmental context to assess whether the drug produced reinforcing effects. The CPP apparatus consisted of a rectangular shuttle box measuring 90 cm in length, 15 cm in width, and 22 cm in height. The box was divided into two equal compartments by a guillotine door. Each compartment had distinct visual and tactile cues: one had white walls and a grid floor, while the other had black walls and a smooth floor. These differences allowed the rats to distinguish between the two environments [2].
The CPP procedure included three phases: preconditioning, conditioning, and postconditioning. During the preconditioning phase, rats were placed in one compartment of the shuttle box and allowed to explore both compartments freely for 15 minutes over three consecutive days. On the third day, the time each rat spent in each compartment was recorded to establish baseline preferences. In the conditioning phase, which lasted four days, rats received alternating injections of FCF or saline. After each injection, they were confined for 15 minutes to one of the compartments. Typically, one compartment was paired with FCF administration and the other with saline. This pairing allowed the rats to associate the drug’s effects with a specific environment [2].
The final phase, postconditioning, occurred on the fifth day. In this phase, the guillotine door was opened, and rats were placed in the initial compartment and allowed to move freely between both compartments for 15 minutes. No drug was administered during this test. The amount of time spent in each compartment was recorded to determine whether the rats developed a preference for the environment previously associated with FCF. An increased time spent in the drug-paired compartment was interpreted as evidence of the drug’s rewarding or reinforcing properties.
Statistical analysis was conducted to evaluate the significance of the findings. For the behavioral sensitization experiment, data for each measured behavior were analyzed using the Student’s t-test to compare differences between the FCF-treated and control groups. For the CPP experiment, a two-way analysis of variance (ANOVA) was used to assess the effects of treatment and conditioning. When significant differences were found, the Newman-Keuls post hoc test was applied to identify specific group differences. Overall, the methods described in this passage outline a well-controlled experimental approach to studying both the behavioral and rewarding effects of repeated fencamfamine exposure in rats, using established behavioral assays and rigorous statistical analysis [2].
Discussion
1) The results of the study conducted by the research team of Ferreira et al demonstrate that FCF significantly reduces Na⁺/K⁺-ATPase activity in the rat striatum through a mechanism involving dopamine signaling, cAMP, and PKA. Multiple lines of experimental evidence support this conclusion. FCF produced a clear dose-dependent inhibition of Na⁺/K⁺-ATPase activity across the tested concentration range of 10–100 µM) The inhibitory effect began at the lowest concentration of 10 µM and increased progressively, reaching a maximal reduction of approximately 51.5% at 100 µM. The calculated IC₅₀ value (the concentration required to inhibit enzyme activity by 50%) was approximately 4.7 × 10⁻⁵ M, indicating moderate potency. Importantly, FCF did not affect Mg-ATPase activity, demonstrating that its effect was selective for Na⁺/K⁺-ATPase rather than causing a general suppression of ATPase enzymes [1].
Time-course experiments revealed that the inhibitory effect of FCF persisted even after the drug was removed. Reduced Na⁺/K⁺-ATPase activity was observed consistently over a 5–60 minute period, indicating that FCF induces a lasting modification of enzyme function rather than a transient interaction. DA, tested at 10 µM, produced a similar degree of inhibition of Na⁺/K⁺-ATPase activity as high-dose FCF at a concentration of 100 µM. This suggests that FCF may act through dopaminergic mechanisms. When FCF and dopamine were applied together, their effects were not additive. The combined treatment did not produce greater inhibition than either drug alone. This nonadditive effect strongly suggests that both compounds act through a shared pathway or mechanism [1].
Both FCF and dopamine significantly increased intracellular levels of cAMP, while having no effect on cGMP levels. This indicates that the signaling pathway involved is specific to cAMP rather than cGMP. The increase in cAMP correlated with the observed decrease in Na⁺/K⁺-ATPase activity, supporting the idea that cAMP mediates the inhibitory effect. Further evidence came from experiments using 8-बromo-cAMP, a cAMP analog. This compound mimicked the effect of FCF, producing a similar reduction in Na⁺/K⁺-ATPase activity without affecting Mg-ATPase. This confirms that activation of cAMP signaling is sufficient to inhibit the enzyme.
To determine whether dopamine receptors were involved, the researchers used selective D1 and D2 receptor antagonists including SCH 23390 and Sulpiride. Pretreatment with either antagonist completely blocked the inhibitory effect of FCF on Na⁺/K⁺-ATPase activity. This indicates that both D1 and D2 dopamine receptors are necessary for FCF’s action. These findings support the idea that FCF increases dopamine signaling, which then activates both receptor subtypes to produce downstream effects.
The involvement of protein kinases was tested using selective inhibitors for PKA and PKG including KT 5720 and KT 5823. Pretreatment with KT 5720 abolished the inhibitory effects of both FCF and 8-बromo-cAMP on Na⁺/K⁺-ATPase activity. In contrast, KT 5823 had no effect on these responses. Additionally, neither inhibitor alone altered enzyme activity, indicating that their effects were specific to blocking the signaling pathway rather than directly affecting the enzyme. These results demonstrate that PKA, but not PKG, is essential for mediating the inhibitory effect of FCF [1].
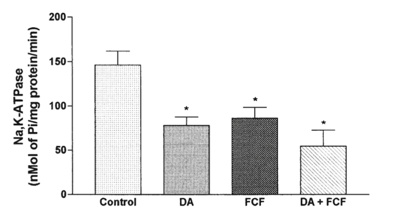
Figure 1: Changes in NA+/K+-ATPase activity in response to DA and FCF in varying concentrations.
Taken together, the results support the following mechanism that FCF enhances dopaminergic signaling likely by increasing dopamine release or blocking reuptake. Additionally, dopamine activates D1 and D2 receptors in the striatum resulting in the increase in intracellular cAMP levels. These increased cAMP levels activate PKA which then phosphorylates components of the Na⁺/K⁺-ATPase system, and ultimately reduces enzyme activity. The lack of involvement of cGMP and PKG further confirms the specificity of the cAMP-PKA pathway.
The key conclusion of this study reports that FCF is a potent inhibitor of Na⁺/K⁺-ATPase in rat striatum, the effects were found to be is dose-dependent, selective, and sustained. Additionally FCF and dopamine were shown to share a common mechanism of action and all inhibitory effects were modulated by an increase in cAMP levels. Both D1 and D2 dopamine receptors were required for this mechanism and while PKA activation was essential, PKG was not involved. Overall, the findings provide strong biochemical evidence that FCF modulates neuronal ion transport through a dopamine-dependent cAMP-PKA signaling cascade, offering insight into its central nervous system effects [1].
2) The study performed by the research team of DeLucia et al presents the key findings and interpretation of experiments examining the behavioral and rewarding effects of repeated FCF administration in rats. The results demonstrate that repeated exposure to FCF produces both behavioral sensitization and an enhanced reinforcing effect, supporting the idea that this psychostimulant engages neural mechanisms similar to those of other addictive drugs [2].
The first set of results focuses on behavioral sensitization, which refers to the progressive intensification of a drug’s effects following repeated use. As described, repeated administration of FCF led to significant increases in sniffing, rearing, and locomotion when compared to the saline-treated control group. These effects were observed both on the first day and after ten consecutive days of treatment, indicating that FCF has strong acute behavioral effects that persist and evolve with repeated exposure. However, when the individual behavioral components were analyzed more closely, a more nuanced pattern emerged. Although overall activity increased, the specific behaviors showed distinct changes over time. In particular, rats treated with FCF exhibited a significant increase in sniffing duration, while simultaneously showing decreases in rearing and locomotion durations. This shift suggests that repeated drug exposure alters not just the intensity but also the pattern of behavior [2].
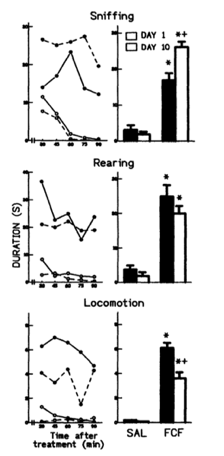
Figure 2: Changes in the duration of sniffing, rearing, and locomotion following repeated exposure to FCF.
These behaviors, sniffing, rearing, and locomotion, are considered mutually exclusive, meaning that an increase in one often corresponds to a decrease in others. Therefore, the observed pattern of increased sniffing with reduced locomotion and rearing reflects a reorganization of behavioral output rather than a simple increase in overall activity. This pattern has been interpreted in prior research as a hallmark of behavioral sensitization, where repeated drug exposure leads to more focused or stereotyped behaviors. Importantly, no significant changes were observed in the saline-treated group between day 1 and day 10, confirming that these effects are specific to FCF and not due to repeated handling or testing [2].
The second major finding relates to the rewarding properties of FCF, assessed using the CPP paradigm. In this test, the amount of time an animal spends in an environment previously paired with drug exposure is used as an indicator of the drug’s reinforcing effects. The results showed that rats treated with FCF for ten consecutive days spent significantly more time in the drug-paired compartment during the postconditioning phase compared to the preconditioning phase. This increase indicates that the animals developed a preference for the environment associated with FCF, demonstrating that the drug has rewarding properties.
Crucially, the increase in time spent in the drug-paired compartment after repeated exposure suggests that the reinforcing effects of FCF were enhanced over time. In other words, repeated administration did not just maintain the drug’s rewarding effects, it intensified them. This phenomenon is consistent with sensitization of the brain’s reward system, where repeated drug use leads to progressively stronger motivational effects. The discussion section places these findings within the broader context of psychostimulant research. The authors conclude that repeated exposure to FCF enhances both behavioral sensitization and the drug’s rewarding effects. These two phenomena are thought to be closely related and may share underlying neural mechanisms [2].
One key mechanism implicated in these effects is the dopaminergic system. Dopamine is a neurotransmitter that plays a central role in motivation, reward, and motor activity. The authors note that brain regions such as the dorsal striatum, including the caudate-putamen and the ventral striatum, particularly the nucleus accumbens, are critically involved in the development and expression of behavioral sensitization. These regions are known to be heavily influenced by dopaminergic signaling and are central components of the brain’s reward circuitry.
Although the precise neural mechanisms underlying FCF-induced sensitization are not fully understood, the findings are consistent with existing theories about how psychostimulants exert their effects. Specifically, it has been proposed that drugs like FCF, amphetamine, cocaine, and morphine produce their reinforcing effects by stimulating the mesocorticolimbic dopamine system. This system is also involved in regulating psychomotor activity, suggesting a shared neural basis for both behavioral activation and reward.
The authors reference the hypothesis that behavioral sensitization and drug reward are mediated by a common mechanism. According to this view, repeated activation of dopaminergic pathways enhances both the motor-stimulating and reinforcing effects of a drug. The results of this study support this idea, as repeated FCF exposure led to both increased behavioral sensitization as seen in altered activity patterns and enhanced place preference indicating stronger reward. Furthermore, the findings are consistent with previous research on other drugs of abuse. Studies have shown that repeated exposure to substances such as amphetamine, cocaine, and morphine also leads to increased rewarding effects over time. This suggests that sensitization of the brain’s reward system is a general feature of addictive drugs, rather than something unique to FCF [2].
The authors conclude that repeated administration of FCF sensitizes the central reward mechanisms in a manner similar to other addictive substances. As a result, the drug produces progressively greater reinforcing effects with repeated use. This has important implications for understanding the potential for abuse and dependence associated with FCF, as well as for broader theories of addiction. In summary, the results demonstrate that repeated FCF exposure leads to significant behavioral changes indicative of sensitization, as well as enhanced rewarding effects as measured by conditioned place preference. These findings support the idea that FCF acts on dopaminergic reward pathways and shares key properties with other psychostimulant drugs of abuse [2].
Disclaimer
**LAB USE ONLY**
*This information is for educational purposes only and does not constitute medical advice. THE PRODUCTS DESCRIBED HEREIN ARE FOR RESEARCH USE ONLY. All clinical research must be conducted with oversight from the appropriate Institutional Review Board (IRB). All preclinical research must be conducted with oversight from the appropriate Institutional Animal Care and Use Committee (IACUC) following the guidelines of the Animal Welfare Act (AWA).
Citations
[1] Pinto Ferreira M, DeLucia R, Luiz Aizenstein M, Glezer I, Scavone C. Fencamfamine modulates sodium, potassium-ATPase through cyclic AMP and cyclic AMP-dependent protein kinase in rat striatum. J Neural Transm (Vienna). 1998;105(6-7):549-560. doi:10.1007/s007020050078
[2] DeLucia R, Planeta CS, Aizenstein ML, Scavone C. Repeated administration intensifies the reinforcing effect of fencamfamine in rats. Gen Pharmacol. 1997;29(2):265-267. doi:10.1016/s0306-3623(96)00414-4
DiEt-Fencamfamin is sold for laboratory research use only. Terms of sale apply. Not for human consumption, nor medical, veterinary, or household uses. Please familiarize yourself with our Terms & Conditions prior to ordering.
| File Name | View/Download |
| 2026-07-09-Umbrella-Labs-DiET-Fencamfamin-Certificate-of-Analysis-COA.pdf |  |
VIEW CERTIFICATES OF ANALYSIS (COA)
Additional information
| Weight | 1 oz |
|---|


